


Abstract
Maize (Zea mays, L.) productivity in sub-Saharan Africa (SSA) remains low, despite breeding efforts spanning across decades. Currently, three-way cross hybrids (TWCH) dominate SSA; however, there is the potential to increase yields by using single-cross hybrids. In this study, five new and four elite CIMMYT lines were inter-mated in a half diallel mating scheme to estimate the combining ability of the lines and to determine the stability of their corresponding 36 single-cross hybrids for grain yield under low-nitrogen stress and optimum growing conditions in Zimbabwe and Zambia. The results revealed that the new inbred line CL121290 showed the highest GCA effects under optimum conditions (1.4 tha−1; p < 0.001) and across sites (0.93 tha−1; p < 0.001). The single-cross hybrids G12 (CML311 × DJL173527) and G16 (DJL173887 × CL1211559) were highly stable and were observed as ideal crosses within both the low-nitrogen and optimal environments. However, G18 (CML311 × DJL173887), which was depicted as ideal genotype under the two management conditions, was an unstable genotype. Hybrid G31 (CML311 × CML312) had the least grain yield under low-nitrogen, optimum and across environments. The hybrid G11 (DJL173527 × CL121290) was the highest yielding genotype amongst the new single-cross hybrids and across environments but was unstable and can be recommended for high potential in environments. Overall, the data demonstrated the potential of single-cross hybrids to supplement TWCH in boosting maize productivity under optimal and nitrogen-stress environments in SSA as well as under other areas with similar climatic conditions in the world.
1. Introduction
Maize (Zea mays L.) is a multi-purpose cereal crop worldwide, where 66% of the produce is used as livestock feed, 20% as direct food for humans, 8% for industrial purposes and 6% is recycled as seed or wasted [1,2]. It is the primary source of calories in sub-Saharan Africa (SSA), contributing about 19% of the calorie intake [3,4]. In the SSA region, maize productivity is limited by multiple factors, such as drought and high temperatures, induced by climate change [5,6,7].
Additionally, a lack of access to resources (e.g., fertilizers, pesticides and irrigation), especially in the small-scale farming sectors, worsens the situation in households that solely depend on maize as a staple crop [8]. Nitrogen (N), phosphorus (P) and potassium (K) are major nutrient requirements for maize productivity; however, N is the most limiting nutrient in tropical soils [8].
Soils in SSA have intrinsically low nitrogen, making maize production unsustainable [9]. Yields in the smallholder farming sector in SSA are low due to low and depleted soil fertility among other factors. Inorganic fertilizer use across SSA is less than economically optimal resulting in low grain yields [10]. Marginal areas are used for maize production by some resource poor farmers, while high value crops take up the more productive lands [11]. As the global population is estimated to double by the year 2050, coupled with the continued decline in land suitable for agriculture [12], there is the need to develop sustainable solutions that can lead to increased maize productivity under these predicted climatic and socio-economic scenarios.
Breeding programs in Africa have traditionally targeted producing TWCH as the final product for the farmer, as opposed to single-cross hybrids that are predominantly grown in some of the world’s largest maize producing countries, such as the USA and China. TWCH are cheap to produce and could be more resilient under the constrained production environments common in SSA (due to some form of genetic buffer effect); although their yield potential is lower than that of the single-cross hybrids [13]. Heterosis is known to be higher in single-cross than in TWCH [14]. One way to increase productivity of maize in SSA may be to switch to the development and extensive deployment of single-cross hybrids that have been so successful in other countries, such as the USA [15].
To be economically viable, parental inbred lines must have desirable characteristics that include not only high seed yield but also good combining ability and yield stability of their hybrid combinations. There is the need for deploying high-yielding, stable (across optimal and marginal growing conditions) and economically viable hybrids for the low-input production systems.
Recently, CIMMYT maize breeders developed inbred lines tolerant to low nitrogen, drought and heat stresses in addition to good per se seed yield, which is an important trait for commercial seed production. Prior to their release as CIMMYT Maize Lines (CMLs), these inbred lines had undergone a series of tests in which their value in maize breeding programs and in commercial seed production systems was evaluated. The selection of a certain hybrid for one (specific adaptation) or many (wide adaptation) environments for grain yield is important.
Grain yield is a quantitatively inherited trait and therefore shows large genotype–environment interactions (GEI) [16], because cultivars grown in different environments differ in performance and stability. The objective of this study was to determine the combining ability of new lines and the stability of their single-cross hybrid combinations for grain-yield performance under optimum and low-nitrogen stress conditions. We hypothesize that some of the new inbred lines can be the parents of high-yielding and stable single-cross hybrids that can complement or replace TWCH to boost the maize productivity under stress and non-stress conditions.
2. Materials and Methods
2.1. Germplasm and Test Sites
A total of nine inbred lines (i.e., four heterotic group A + five heterotic group B) adapted to the mid-altitudes of SSA: five new and four CMLs (Table 1) were crossed following the Griffing diallel Method 4 (half diallel) mating scheme [17]. The assumptions of the method include: (i) diploid segregation; (ii) homozygous parents; (iii) no multiple allelism; (iv) there is no difference between reciprocal crosses; (v) independent action of non-allelic genes in the diallel cross; and (vi) genes independently distributed between the parents.
Table 1.
Maize inbred line parents for the partial diallel crosses.
CIMMYT maize inbred lines were classified into different heterotic groups based on the predominant racial origin of the source population and combining ability with established heterotic testers as either Tuxpeño (Group A; e.g., Population 21) or non-Tuxpeño (Group B; e.g., Population 32) [18]. The crosses were made at Muzarabani station; 16°34′ S; 31°08′ E; 360 masl in Zimbabwe, during the winter season (May to October 2017).
The CMLs are, per CIMMYT standards, released and publicly available inbred lines already used as the parents of commercialized hybrids and widely used for breeding [19]. The resultant 36 single-cross hybrids and four single-cross hybrid checks (medium maturing yellow maize- SC608; medium maturing white maize- SC633; late maturing white maize- SC727 and CZH15429) were evaluated at eight sites during 2018 and 2019 summer seasons in Zimbabwe and Zambia (Table 2). The checks were chosen on the premise that they are single-cross hybrids currently marketed widely to farmers in the region.
Table 2.
Characteristics of the testing sites used to evaluate single-cross hybrids in Zimbabwe and Zambia in 2018 and 2019.
2.2. Experimental Design
The experiment was laid out in an alpha (0, 1) lattice design [20] with two replications at each site. The plot size was one-row 4 m long with an inter-row spacing of 0.75 m and 0.25 m between plants in a row. Two seeds were sown per hill and later thinned to one plant per station at three weeks after emergence for a final density of approximately 55, 000 plants ha−1.
2.3. Management
The hybrids were subjected to two treatments: low-nitrogen stress and optimum conditions (Table 2). The low-N experiments were established at three sites in fields that were depleted of nitrogen by continuously planting maize without adding any inorganic or organic nitrogen fertilizer across a period of four cropping seasons. Locations traditionally used for low-nitrogen screening in Zimbabwe are those with nitrate-N levels below 20 ppm [21]. At the end of each season, all the crop residues were removed from the field [22]. In the low-nitrogen trials, only phosphorus and potassium fertilizers were applied. The five optimum trials were managed following the recommended agronomic practices, including supplementing rainfall with irrigation whenever necessary and also applying the recommended doses of basal and top-dressing fertilizers [23].
2.4. Data Collection
Quantitative traits, such as the grain yield, plant height, days to anthesis, days to silking, ear height and ears per plant, were recorded. The grain weight and grain moisture (expressed as a percentage) were recorded at harvest and used to calculate the grain yield (shelled grain weight per plot adjusted to 12.5% grain moisture converted to tons per hectare).
2.5. Statistical Analysis
ANOVA for the grain yield for each environment and combined ANOVA were computed using restricted maximum likelihood (REML) analysis using linear mixed models in the GenStat software 14th edition (VSN International, England, UK) [24]. Entries were considered fixed effects, whereas sites were considered random effects. The significance of different items in the ANOVA was tested using the F statistic (p < 0.05), which is the ratio of the sum of mean squares to the mean square error. ANOVA for a single environment (i.e., site) was done according to the linear model by Barreto et al. [25] as follows:
where Yijk is the response variable/trait, e.g., yield, µ is the grand mean, rj BK is the effect of the kth block nested in the ith replication, k represents 1, 2, 3, 4 and 5, blocks, and i stands for 1, 2 and 3 replications.
Yijk = μ + ri Bk + Ej + εijk
A combined ANOVA across the eight sites was also done according to the linear model by Barreto et al. [25] as follows:
where Yijkl is the response variable/trait, µ is the grand mean, rj BK is the effect of the kth block nested in the jth replication, k represents 1, 2, 3, 4 and 5, blocks, j represents 1, 2 and 3 replications, Li is the effect of ith location, i represents 1, 2 and 3 locations, El is the effect of the lth entry and l represents 1, 2, 3, 4, …, 25 entries, ELil is the interaction effect of the lth entry and the ith location and εijkl is the experimental error.
Yijkl = μ + rj Bk + Li + El + [EL]il + εijkl
The narrow-sense and broad-sense heritability were both estimated for comparison sake and because it is restrictive to predict performance of a hybrid using GCA of an inbred line under low-nitrogen stress. The broad-sense heritability (H) was calculated as the ratio of genotypic variance to phenotypic variance [26] as follows:
where is and genotypic variance and is the phenotypic variance.
The narrow-sense heritability (h2) was calculated using the formula given by Hallauer and Miranda [27].
where is the environmental variance, is the mean squares of the general combining ability and is the mean squares of the specific combining ability.
The grain yield data of hybrids was subjected to Griffing’s [17], Method 4 and Model 1 analysis using the CIMMYT AGD-R 4.0 software [CIMMYT Biometrics & Statistics Unit, Mexico]; [28]. The diallel analysis model was as follows:
where, xij is the mean of i × jth genotype (g) over kth Environments (E), μ is the population mean, gi and gj are the GCA effects, sij are the SCA effects such that sij = sji (thus, assuming absence of reciprocal effects) and eijk is the random error term. Ekgi, Ekgj and ESij are GCA × Environment and SCA × Environment interaction effects, respectively.
xij = µ + gi + gj + sij + Ek + Ekgi + Ekgj + ESij + eijk
To identify the highest-yielding and stable single-cross hybrids under managed low-nitrogen and optimal conditions, the genotype main effect (G) and genotype-by-environment (G × E) interaction (GGE) biplot analysis [29] was performed in GenStat 14th edition [24]. GGE biplot analysis was also performed in order to identify the best suited genotypes within stress (i.e., low nitrogen) and non-stress (i.e., optimal) conditions. The GGE biplots provides comprehensive visual information, and its advantage over regression is that it is faster and easier to interpret [30].
It also removes the large environmental effect (E) not necessary for genotype evaluation and keeps only G and G × E, which are more pertinent for making useful genotype evaluation and selection decisions [31]. Stability analysis was necessitated by the presence of significant crossover interactions effects between the crosses and the sites observed under both the stress and non-stress environments (see Table 3).
Table 3.
Analysis of variance for grain-yield performance of half diallel crosses evaluated during the 2018 and 2019 summer seasons in Zimbabwe and Zambia.
3. Results
3.1. F1 Hybrid Performance and Combining Ability Effects
The genotypes’ general combining ability (GCA) and specific combining ability (SCA) mean squares were significant (p < 0.001) for grain yield under optimal conditions and across sites (Table 3). The genotype–environment interaction (GEI) was significant for grain yield under low-nitrogen stress (p < 0.05), optimal conditions (p < 0.01) and across sites (p < 0.001). The GCA × site interaction effects were significant under optimal conditions and across sites. The GCA mean squares values were lower compared to the SCA mean squares under managed low-nitrogen stress, optimal conditions and across sites.
Both the narrow-sense heritability (h2 = 2%) and broad-sense heritability (H2 = 48%) estimates for grain yield under managed low-nitrogen stress conditions were lower than those observed under optimal conditions, i.e., 51% and 88%, respectively (Table 3). A breeder cannot predict hybrid performance under low-nitrogen stress using GCA. There is a huge difference between the narrow-sense and broad-sense heritability because non-additive gene action (SCA) is added to the performance of grain yield under low nitrogen. The narrow-sense heritability for grain yield is generally low under stress, ranging between 5% and 10% [32].
The new inbred line P5 (CL1212902) had the highest and significant GCA effects for grain yield under optimal conditions and across sites, whereas P2 (DJL173527) was the best general combiner for grain yield under low-nitrogen conditions (Table 4). Elite inbred line parents that showed positive and significant GCA effects for grain yield were found for CML543 and CML566.
Table 4.
The general combining ability (GCA) effects of new and elite CIMMYT lines evaluated under low-nitrogen and optimal conditions in Zimbabwe and Zambia during the 2018 and 2019 summer seasons.
3.2. Potential of the New Inbred Line Parents for Grain-Yield Performance in Single-Cross Hybrid Combinations
Table 5 and Table 6 show the grain-yield performance and specific combining ability values of 36 new single-cross hybrids under low-nitrogen, optimal conditions and across environments. The best three specific combiners for grain yield (GY) performance under optimal management conditions were the genotypes G12, G11 and G35. Under low-nitrogen stress conditions, the best three specific combiners were G16, G19 and G12. In addition, across low-nitrogen and optimal conditions, the best were G18 and G16 (Table 5).
Table 5.
The specific combining ability (SCA) effects of new and elite CIMMYT lines evaluated under low-nitrogen and optimal conditions in Zimbabwe and Zambia during the 2018 and 2019 summer seasons.
Table 6.
The grain-yield performance of the 36 diallel crosses and the four check hybrids evaluated under low-nitrogen and optimal conditions in Zimbabwe and Zambia during the 2018 and 2019 summer seasons.
New inbred line parents P2 and P5 showed the highest potential in single-cross hybrid combinations under optimal conditions, whereas P2, P3 and P4 indicated high potential across the low-nitrogen and optimal conditions. Under low-nitrogen conditions, G16 and G12 performed better than the other three checks (G40, G37 and G38). Under optimum conditions G11 and G29 outperformed all the four single-cross hybrid checks (Table 6).
3.3. Stable High Yielding Single-Cross Hybrids under Low-Nitrogen Stress and Optimal Conditions
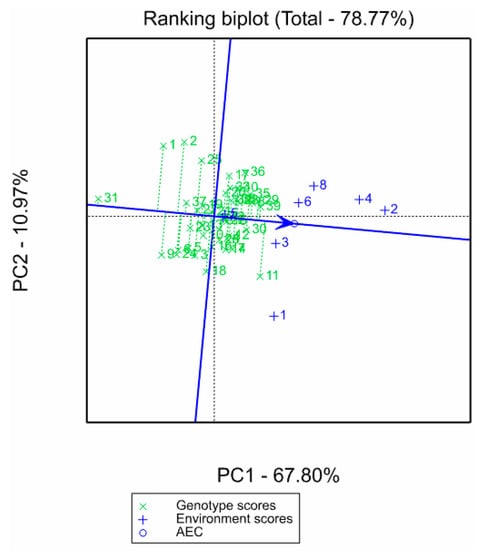
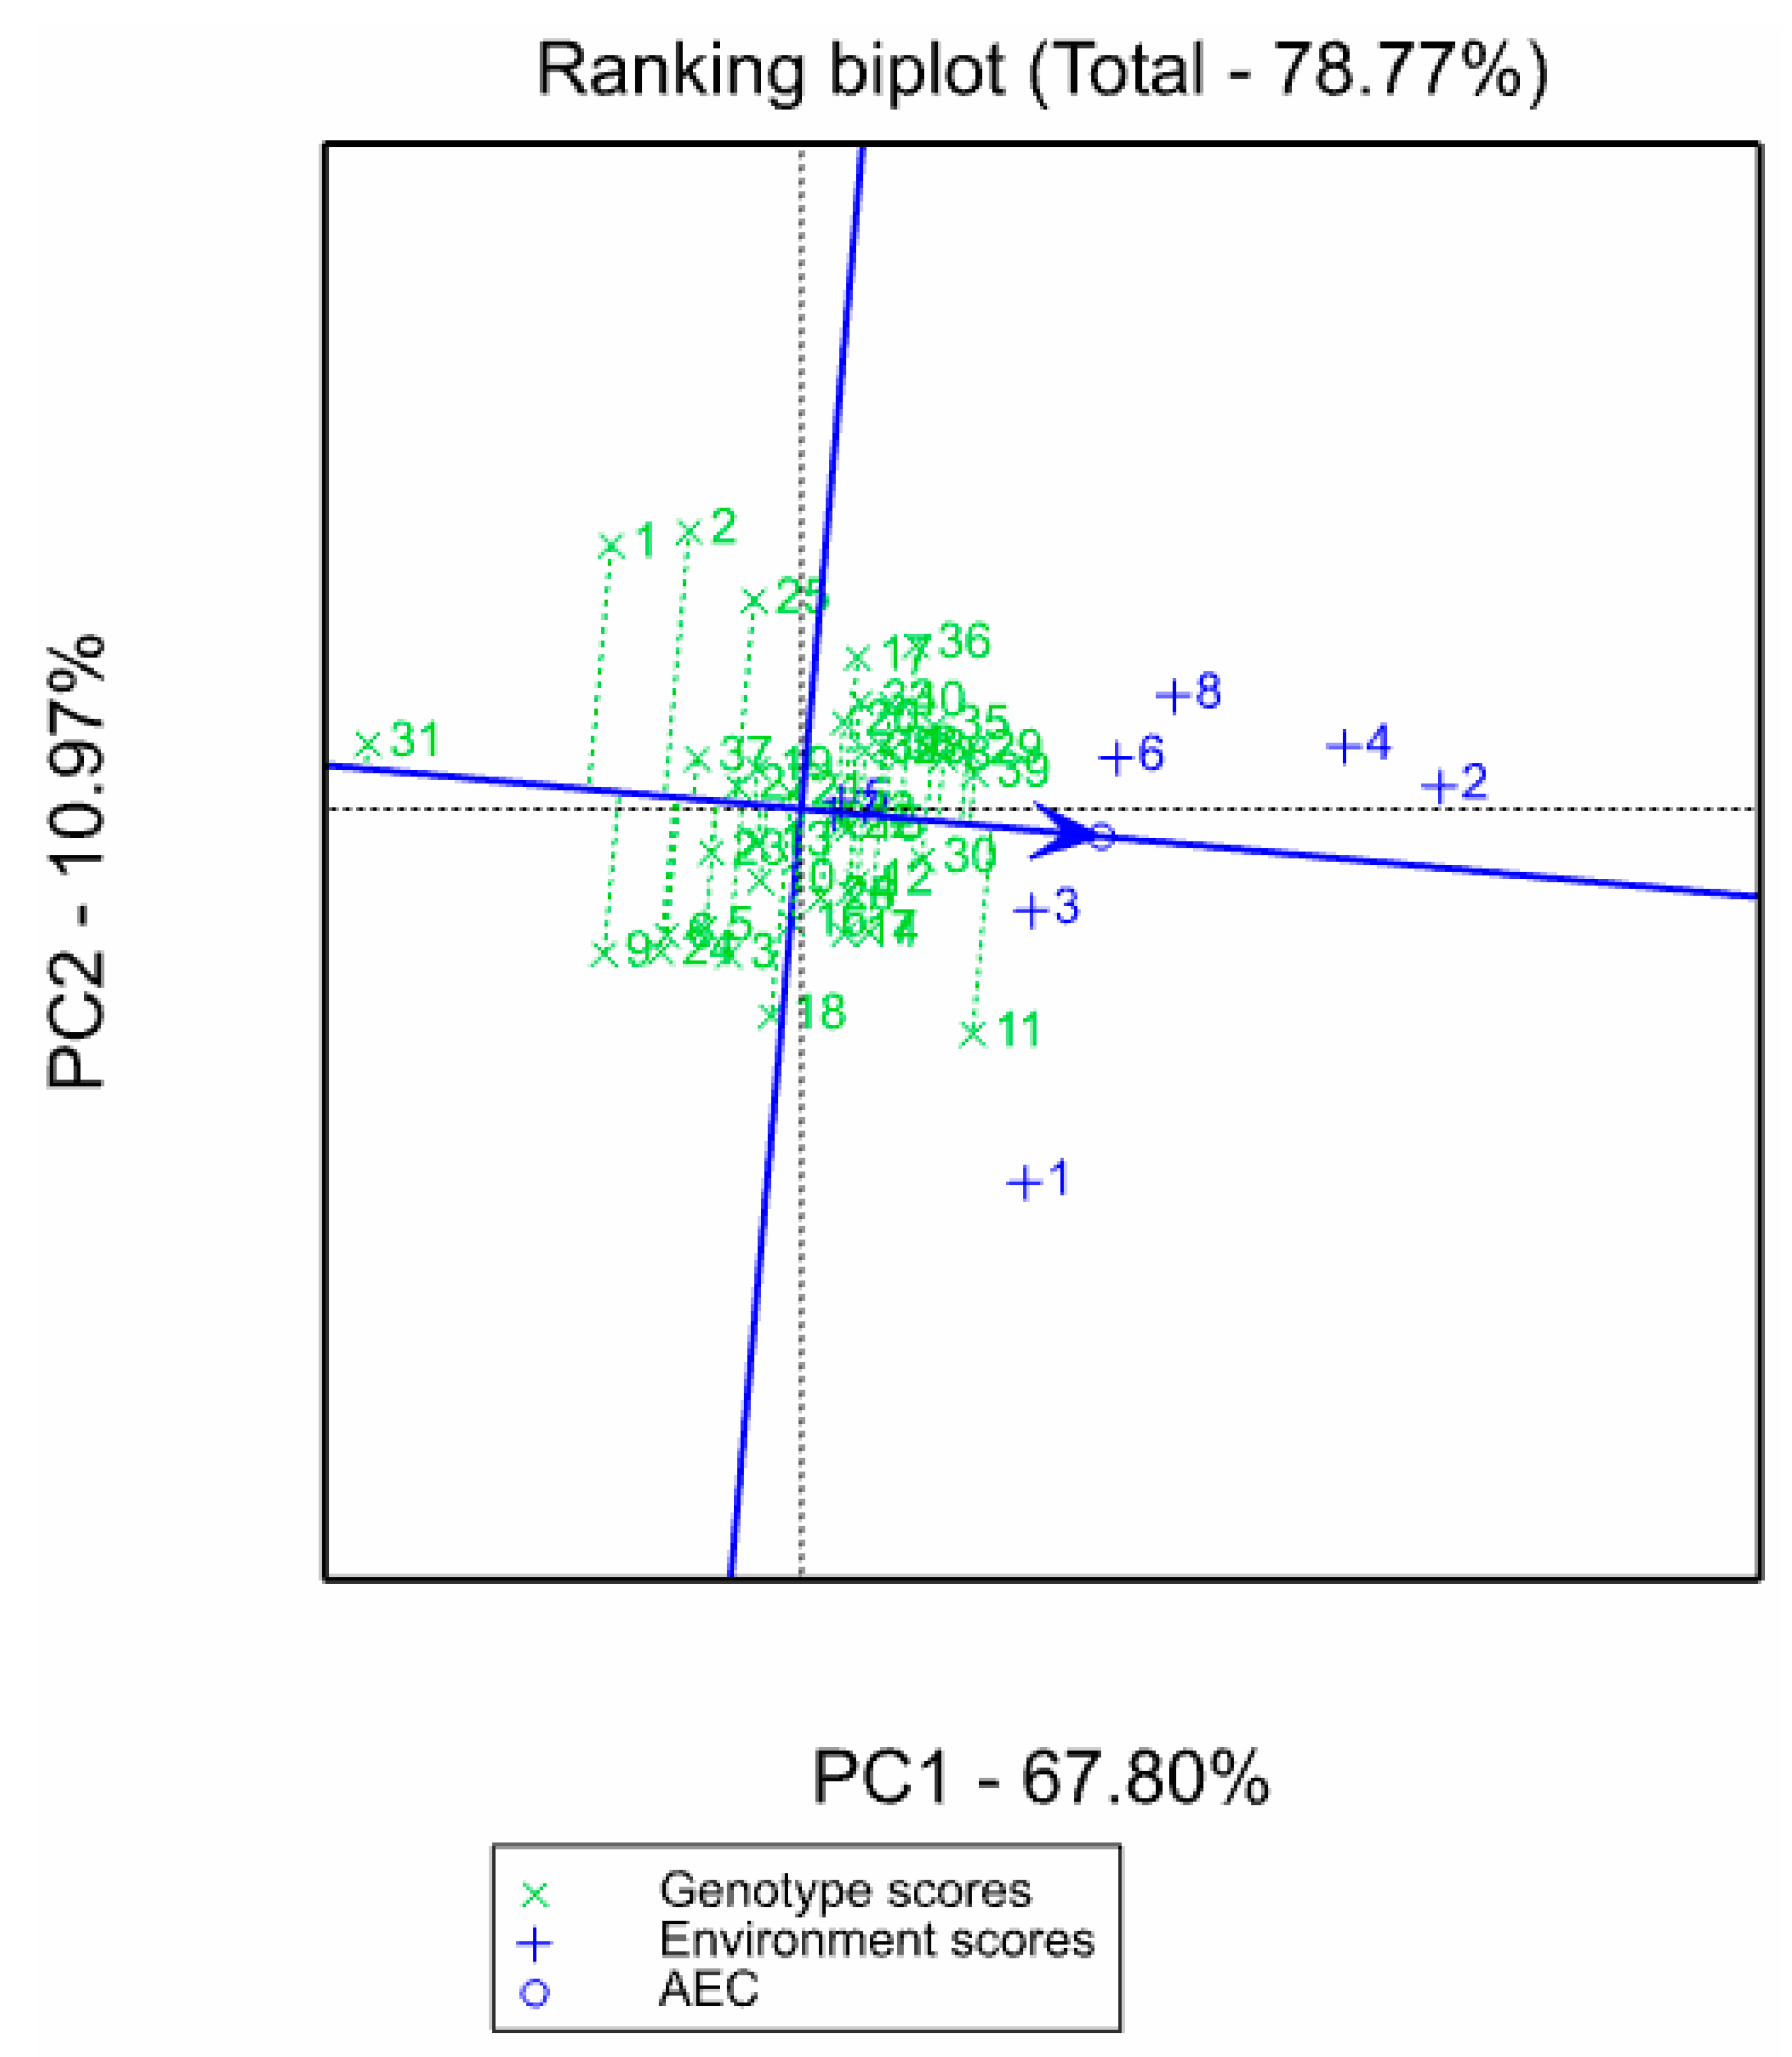
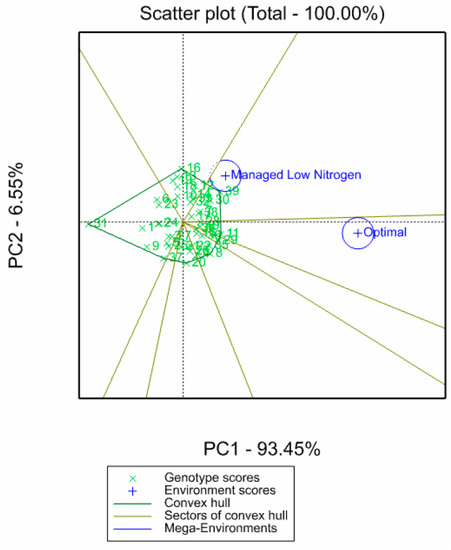
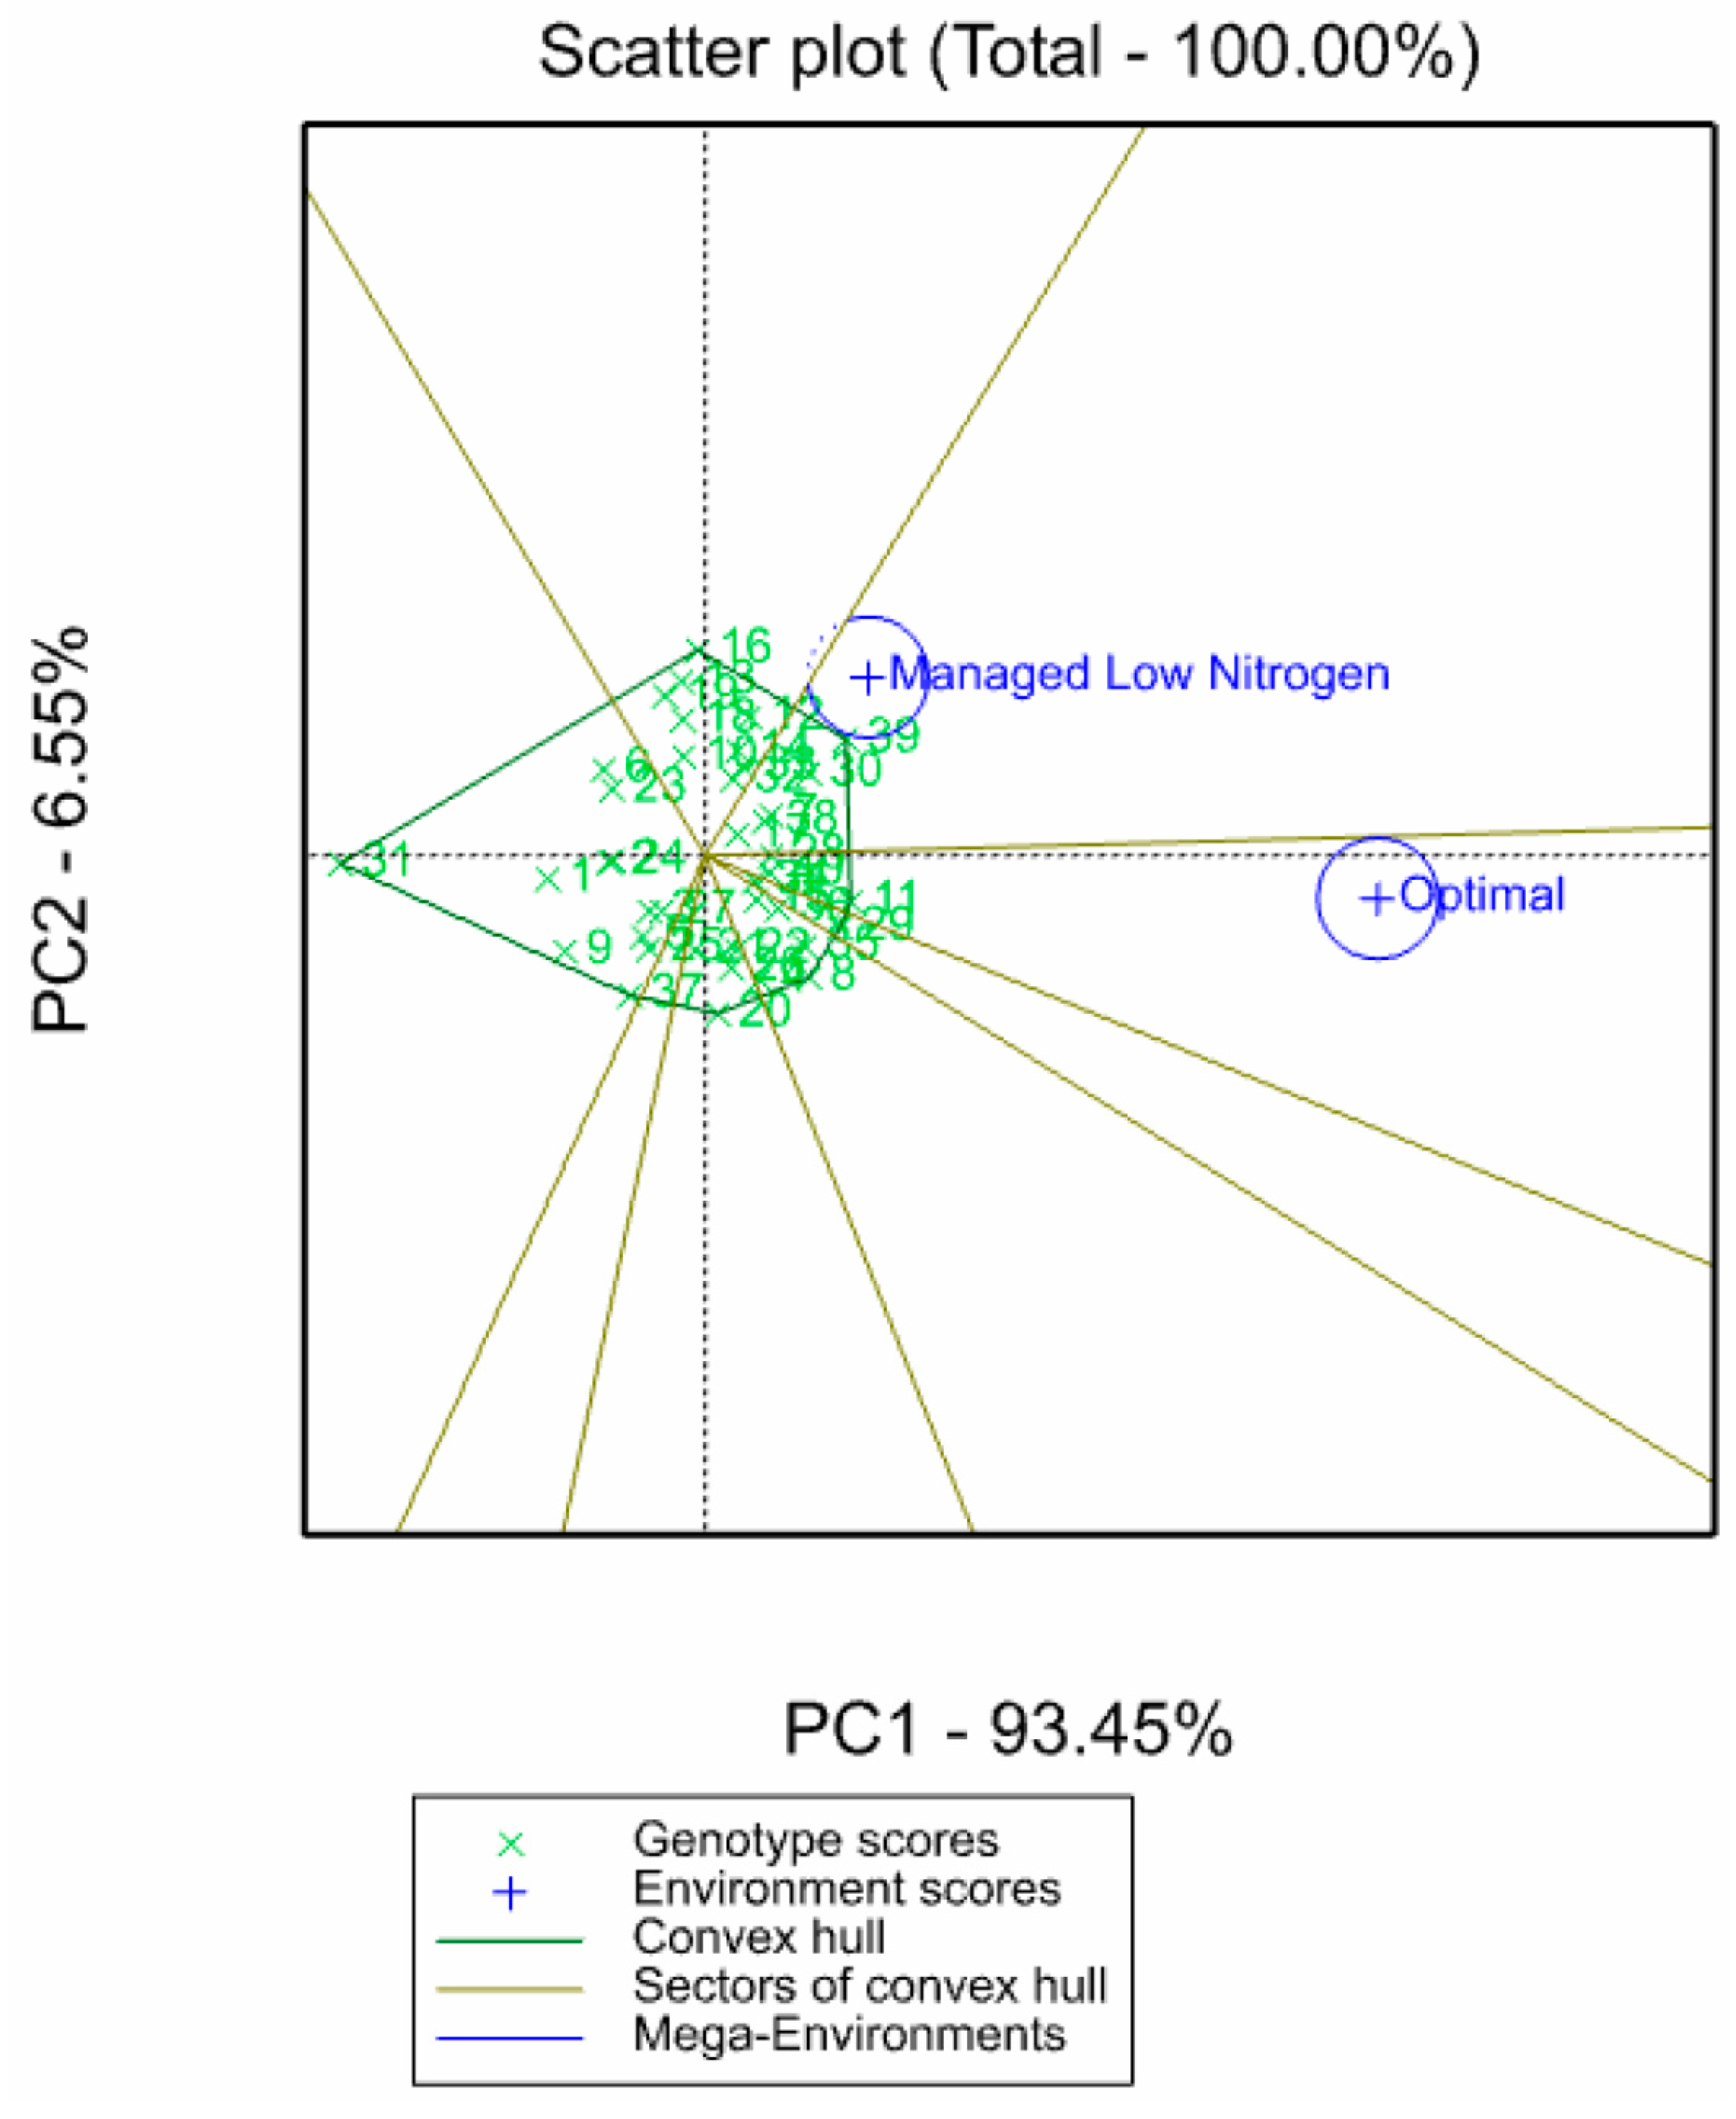
Figure 1 show that G11 (P5 × P2) was highly unstable though it was the highest yielding genotype amongst the new single-cross hybrids as well as the checks. G11 was also identified as the most suited genotype under optimal conditions, whereas genotype 39 (Check 3) was predicted to be the most ideal under low-nitrogen conditions (Figure 2). G12 (P6 × P2) and G16 (P4 × P3) across low-nitrogen stress and optimal growing conditions were also observed to be highly stable. However, genotype 18 (P6 × P3), which was depicted as an ideal genotype under the two management conditions, was unstable for grain-yield performance (Figure 1).
Figure 1.
Biplot of the average environment coordination (AEC) view showing the mean performance and stability of diallel cross genotypes (1–36) and checks (37–40) across eight low-nitrogen and optimal sites in Zimbabwe and Zambia.
Figure 2.
Biplot of the average environment coordination (AEC) view showing the diallel cross genotypes (1–36) and checks (37–40) specifically adapted to low-nitrogen and optimally managed sites in Zimbabwe and Zambia.
4. Discussion
In the current study, we hypothesized that some of the new inbred lines could potentially contribute to the development of high yielding and stable single-cross hybrids that can supplement three-way hybrids in boosting maize productivity in SSA. The significant GCA and SCA effects across environments indicate the relative changes in combining ability effects across management levels [22].
The non-significant GCA × site interaction effects on the grain-yield performance observed under low-nitrogen stress conditions meant that low-N sites were similar, and this observation was inconsistent with the findings of Ertiro et al. [33] where low-N sites were significantly different. The significant estimates of the GCA and SCA variances suggested the importance of both additive and non-additive gene actions for the expression of grain yield [34].
However, the additive genetic effects appeared to be less important than the non-additive genetic effects for grain-yield performance under both optimal and low-nitrogen stress conditions. The best hybrids under both conditions had at least one parent with highly significant and positive GCA effects for grain yield, and this concurs with the observations of Makumbi et al. [35]. In a separate study by San Vicente et al. [36], a greater relative importance of non-additive genetic effects compared with additive genetic effects for grain-yield performance among the white endosperm maize population was also reported.
Breeding programs in Africa are now considering single-cross hybrids as a way of increasing maize productivity. Single-cross hybrids are considered unstable in the adverse stress conditions commonly present in SSA, and the seeds are expensive because of the costs of producing seeds [13]. Although this narrative can be proven to be true for most of the commercial varieties in the market, our results demonstrated that the new stress-tolerant single-cross hybrids can be stable across environments.
The new inbred lines used in this study were chosen because they are known to have high per se grain yield, which is a favorable trait in minimizing seed production cost. For instance, the new inbred line P5 (CL1212902) showed the highest and significant GCA effects for grain yield across environments. The new inbred lines P2 and P5 were involved in the most high-yielding single-cross hybrids (G11, G29 and G30) across environments. The identified stable single-cross hybrids (G12 and G16) were more stable than the commercial hybrids used in this study under optimum and low-nitrogen-stress environments. This observation may suggest that single-cross hybrids may potentially complement the TWCH that are predominantly used in SSA.
Something important to note from these results is that high yielding and/or stable single-cross hybrid cannot only be expected across heterotic groups as it is also possible to have them within the same heterotic group, such as in the case of inbred lines P6 (CML 311) and P2 (DJL173527) (both in heterotic group A) as well as P4 (CL1211559) and P3 (DJL173887) (both in heterotic group B). These inbred lines were also important in specific combinations as parents of single-cross hybrids with highly significant positive SCA values in several instances.
They were also involved in single-crosses with high stability. Pedigree starts are developed from high potential lines within the same heterotic groups (P6 and P2) can potentially contribute to the development of new high yielding heterotic group A inbred lines combining tolerance to low-N and high-grain yield under stress and non-stress environments. Likewise, P4 and P3 can potentially contribute to the development of new heterotic group B inbred lines that are also adapted under low-nitrogen conditions combining tolerance to low N and high-grain yield under low-N and optimal growing conditions.
It is important to mention that the identified superior new low-N-stress-tolerant inbred lines (P2, P3, P4, P5 and P6) can be deployed as parents in crosses targeted at creating new populations for the development of other new stress-tolerant lines. The identified best specific combinations, G12 (P6 × P2) and G16 (P3 × P4), which were highly stable across optimal and marginal growing conditions, should be subjected to further evaluations, particularly under farmer management conditions to generate more supporting data for the release process as commercial varieties. In conclusion, the results revealed that some of the new inbred lines can potentially contribute to the development of high yielding and stable single-cross hybrids that can supplement three-way hybrids in boosting maize productivity in SSA.
Author Contributions
F.M. performed the research and wrote the manuscript; C.M. supervised the field research work; S.D. and E.G. edited the manuscript; U.M. was the administrative supervisor for the research; C.N.K. performed data analysis and co-wrote the manuscript. All authors have read and agreed to the published version of the manuscript.
Funding
This study was funded by the Stress Tolerant Maize for Africa (STMA, Grant no. OPP1134248), project funded by the Bill & Melinda Gates Foundation and USAID and the CGIAR maize research program.
Data Availability Statement
Not applicable.
Acknowledgments
The authors thank Kelvin Simpasa, Irene Viola, Toverengwa Chitana, Alex Chikoshana, Stanley Gokoma and Semai Viola for their technical assistance at the various experimental sites used in the study. We also acknowledge Seed Co., Zimbabwe for their research support at their experimental sites in Zambia and Zimbabwe.
Conflicts of Interest
The authors declare no conflict of interest.
References
- Aslam, M.; Cengiz, R. Effects of Drought on Maize. In Drought Stress in Maize (Zea mays L.); Springer International Publishing: Cham, Switzerland, 2015; pp. 5–17. [Google Scholar]
- Doswell, C. Maize in the Third World; CRC Press: Boca Raton, FL, USA, 2019. [Google Scholar]
- Ekpa, O.; Palacios-Rojas, N. Sub-Saharan African maize-based foods: Technological perspectives to increase the food and nutrition security impacts of maize breeding programmes. Glob. Food Secur. 2018, 17, 48–56. [Google Scholar] [CrossRef] [Scilit]
- Lydonn. Available online: https://www.world-grain.com/ (accessed on 28 August 2018).
- Nelimor, C.; Badu-Apraku, B. Phenotypic Characterization of Maize Landraces from Sahel and Coastal West Africa Reveals Marked Diversity and Potential for Genetic Improvement. J. Crop Improv. 2019, 34, 122–138. [Google Scholar] [CrossRef] [Scilit]
- Bradshaw, C.D.; Pope, E.; Kay, G.; Davie, J.C.; Cottrell, A.; Bacon, J.; Cosse, A.; Dunstone, N.; Jennings, S.; Challinor, A.; et al. Unprecedented climate extremes in South Africa and implications for maize production. Environ. Res. Lett. 2022, 17, 084028. [Google Scholar] [CrossRef] [Scilit]
- Ortiz-Bobea, A.; Ault, T.R.; Carrillo, C.M.; Chambers, R.G.; Lobell, D.B. Anthropogenic climate change has slowed global agricultural productivity growth. Nat. Clim. Chang. 2021, 11, 306–312. [Google Scholar] [CrossRef] [Scilit]
- Badu-Apraku, B.; Fakorede, M.A.B. Maize in Sub-Saharan Africa: Importance and Production Constraints. In Advances in Genetic Enhancement of Early and Extra-Early Maize for Sub-Saharan Africa; Springer: Cham, Switzerland, 2017. [Google Scholar]
- Dakora, F.D.; Keya, S.O. Contribution of legume nitrogen fixation to sustainable agriculture in Sub-Saharan Africa. Soil Biol. Biochem. 1997, 29, 809–817. [Google Scholar] [CrossRef] [Scilit]
- Ricker-Gilbert, J. Inorganic fertilizer use among smallholder farmers in Sub-Saharan Africa: Implications for input subsidy policies. In The Role of Smallholder Farms in Food and Nutrition Security; Springer: Cham, Switzerland, 2020. [Google Scholar] [CrossRef] [Scilit]
- Masuka, B.; Magorokosho, C. Gains in Maize Genetic Improvement in Eastern and Southern Africa: II. CIMMYT Open-Pollinated Variety Breeding Pipeline. Crop Sci. 2017, 57, 180. [Google Scholar] [CrossRef] [Scilit]
- Grafton, R.; Williams, Q.J.; Jiang, Q. Food and Water Gaps to 2050: Preliminary Results from the Global Food and Water System (GFWS) Platform. Food Secur. 2015, 7, 209–210. [Google Scholar] [CrossRef] [Scilit]
- MacRoberts, J.; Setimela, P.S. Maize Hybrid Seed Production Manual. Handbook. 2014, pp. 27–31. Available online: https://excellenceinbreeding.org/sites/default/files/manual/98078.pdf (accessed on 19 August 2021).
- Eberhart, S.A. Theoretical relations among single, three-way and double-cross hybrids. Int. Biom. Soc. 1964, 20, 522–539. [Google Scholar] [CrossRef] [Scilit]
- Troyer, A.F. Background of U.S hybrid corn II: Breeding, climate, and food. Crop Sci. 2004, 44, 370–380. [Google Scholar] [CrossRef] [Scilit]
- Dari, S.; Macrobert, J. Effect of the fewbranched-1 (Fbr1) tassel mutation on performance of maize inbred lines and hybrids evaluated under stress and optimum environments. Maydica 2017, 12, 62. [Google Scholar]
- Griffing, B. Concept of General and Specific Combining Ability in Relation to Diallel Crossing Systems. Austrialian J. Biol. Sci. 1956, 9, 463–493. [Google Scholar] [CrossRef] [Scilit]
- Wu, Y.; San Vicente, F.; Huang, K.; Dhliwayo, T.; Costich, D.E.; Semagn, K.; Sudha, N.; Olsen, M.; Prasanna, B.M.; Zhang, X.; et al. Molecular characterization of CIMMYT maize inbred lines with genotyping-by-sequencing SNPs. Theor. Appl. Genet. 2016, 129, 753–765. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Semagn, K.; Magorokosho, C. Molecular characterization of diverse CIMMYT maize inbred lines from eastern and Southern Africa using single nucleotide polymorphic markers. BMC Genom. 2012, 13, 113. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Patterson, H.D.; Williams, E.R.; Hunter, E.A. Block Designs for Variety Trials. J. Agric. Sci. (Camb.) 1978, 90, 395–400. [Google Scholar] [CrossRef] [Scilit]
- Arisede, C.; Mainassara, Z.A.; Jill, C.; Amsal, T.; Cosmos, M.; Bish, D.; Benhildah, M.; Mike, O.; Maruthi, P.B. Low-N stress tolerant maize hybrids have higher fertilizer N recovery efficiency and reduced N-dilution in the grain compared to susceptible hybrids under low N conditions. Plant Prod. Sci. 2020, 23, 417–426. [Google Scholar] [CrossRef] [Scilit]
- Tapera, T. Expression of Tolerance to Drought and Low Nitrogen Levels in Maize Inbred Lines and Hybrids in Southern Africa. Ph.D. Thesis, University of the Free State, Bloemfontein, South Africa, 2017; p. 36. [Google Scholar]
- Banziger, M.; Setimela, P. Breeding for Improved Abiotic Stress Tolerance in Maize Adapted to Southern Africa. Agric. Water Manag. 2006, 8, 212–214. [Google Scholar] [CrossRef] [Scilit]
- VSN International. GenStat for Windows, 14th ed.; VSN International: Hemel Hempstead, UK, 2011. [Google Scholar]
- Barreto, H.J.; Edmeades, G.O. The Alpha Lattice Design in Plant Breeding and Agronomy: Generation and Analysis. CIMMYT, Mexico DF (Mexico) [Corporate Author, Physics]. 1997. Available online: https://www.semanticscholar.org/paper/The-alpha-lattice-design-in-plant-breeding-and-and-Barreto-Edmeades/65d3efaaaee5396eef88d580c2799c5b448df6d2 (accessed on 19 August 2021).
- Singh, R.K.; Chaudhary, B.D. Biometrical Methods in Quantitative Genetic Analysis; Kalyani Publishers: New Delhi, India, 1979. [Google Scholar]
- Hallauer, A.R.; Miranda, J.B. Quantitative Genetics in Maize Breeding, 2nd ed.; Iowa State University Press: Ames, IA, USA, 1988. [Google Scholar]
- Rodriguez, F.; Alvarado, G. AGD-R (Analysis of Genetic Designs with R for Windows) (version 3.0). CIMMYT Res. Data Softw. Repos. Netw. 2015, 12, 53. [Google Scholar]
- Yan, W.; Kang, M.S. GGE biplot vs. AMMI analysis of genotype-by-environment data. Crop Sci. 2007, 47, 643–655. [Google Scholar] [CrossRef] [Scilit]
- Meseka, S.K.; Menkir, A.; Ibrahim, A.E.S. Yield potential and yield stability of maize hybrids selected for drought tolerance. J. Appl. Biosci. 2008, 3, 82–90. [Google Scholar]
- Dehghanpour, Z.; Ehdaie, B. Stability of general and specific combining ability effects for grain yield in elite Iranian maize inbred lines. J. Crop Improv. 2013, 27, 137–152. [Google Scholar] [CrossRef] [Scilit]
- Dabholkar, A.R. Elements of Biometrical Genetics; Concept Publishing Company: New Delhi, India, 1992; p. 166. [Google Scholar]
- Ertiro, B.T.; Beyene, Y. Combining ability and testcross performance of drought-tolerant maize inbred lines under stress and non-stress environments in Kenya. Plant Breed. 2017, 136, 197–205. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Talukder, M.Z.A.; Karim, A.S. Combining ability and heterosis on yield and its component traits in maize (Zea mays L.). Bangladesh J. Agric. Res. 2016, 41, 565–577. [Google Scholar] [CrossRef] [Scilit]
- Makumbi, D.; Betrán, J.F. Combining ability, heterosis and genetic diversity in tropical maize (Zea mays L.) under stress and non-stress conditions. Euphytica 2011, 180, 143–162. [Google Scholar] [CrossRef] [Scilit]
- San Vicente, F.; Bejarano, A. Analysis of diallel crosses among improved tropical white endosperm maize populations. Maydica 1998, 43, 147–153. [Google Scholar]

Publisher’s Note: MDPI stays neutral with regard to jurisdictional claims in published maps and institutional affiliations. |
© 2022 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).